

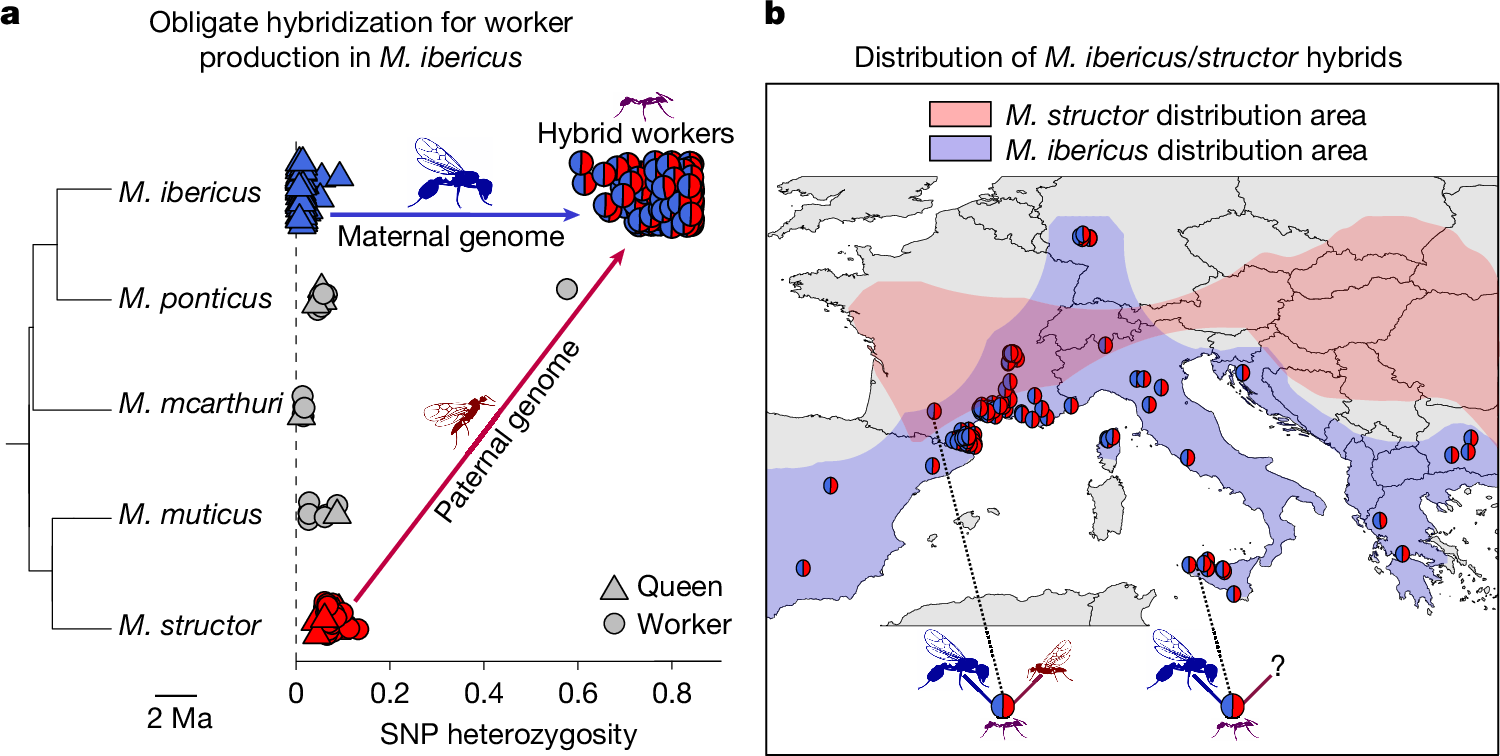
Living organisms are assumed to produce same-species offspring1,2. Here, we report a shift from this norm in Messor ibericus, an ant that lays individuals from two distinct species. In this life cycle, females must clone males of another species because they require their sperm to produce the worker caste. As a result, males from the same mother exhibit distinct genomes and morphologies, as they belong to species that diverged over 5 million years ago. The evolutionary history of this system appears as sexual parasitism3 that evolved into a natural case of cross-species cloning4,5, resulting in the maintenance of a male-only lineage cloned through distinct species’ ova. We term females exhibiting this reproductive mode as xenoparous, meaning they give birth to other species as part of their life cycle.
Sex Redefined: The Idea of 2 Sexes Is Overly Simplistic
Biologists now think there is a larger spectrum than just binary female and male
A common red algal origin of the apicomplexan, dinoflagellate, and heterokont plastids
The discovery of a nonphotosynthetic plastid in malaria and other apicomplexan parasites has sparked a contentious debate about its evolutionary origin. Molecular data have led to conflicting conclusions supporting either its green algal origin or red algal origin, perhaps in common with the plastid of related dinoflagellates. This distinction is critical to our understanding of apicomplexan evolution and the evolutionary history of endosymbiosis and photosynthesis; however, the two plastids are nearly impossible to compare due to their nonoverlapping information content. Here we describe the complete plastid genome sequences and plastid-associated data from two independent photosynthetic lineages represented by Chromera velia and an undescribed alga CCMP3155 that we show are closely related to apicomplexans. These plastids contain a suite of features retained in either apicomplexan (four plastid membranes, the ribosomal superoperon, conserved gene order) or dinoflagellate plastids (form II Rubisco acquired by horizontal transfer, transcript polyuridylylation, thylakoids stacked in triplets) and encode a full collective complement of their reduced gene sets. Together with whole plastid genome phylogenies, these characteristics provide multiple lines of evidence that the extant plastids of apicomplexans and dinoflagellates were inherited by linear descent from a common red algal endosymbiont. Our phylogenetic analyses also support their close relationship to plastids of heterokont algae, indicating they all derive from the same endosymbiosis. Altogether, these findings support a relatively simple path of linear descent for the evolution of photosynthesis in a large proportion of algae and emphasize plastid loss in several lineages (e.g., ciliates, Cryptosporidium , and Phytophthora) .

Termite
Termites are a group of eusocial insects which consume a variety of decaying plant material, generally in the form of wood, leaf litter, and soil humus. They are distinguished by their beaded (moniliform) antennae and the soft-bodied, unpigmented worker caste for which they have been commonly termed "white ants"; however, they are not ants but highly derived cockroaches; they are genetically closer to some cockroach groups than these are to other cockroaches. About 2,997 extant species are currently described, 2,125 of which are members of the family Termitidae.

Social Insects : Ecology and Behavioural Biology
1 online resource; Here is a guide to the ecology of social insects. It is intended for general ecologists and entomologists as well as for undergraduates and those about to start research on social insects; even the experienced investigator may find the comparison between different groups of social insects illuminating. Most technical terms are translated into common language as far as can be done without loss of accuracy but scientific names are unavoidable. Readers will become familiar with the name even though they cannot visualize the animal and could reflect that only a very few of the total species have been studied so far! References too are essential and with these it should be possible to travel more deeply into the vast research literature, still increasing monthly. When I have cited an author in another author's paper, this implies that I have not read the original and the second author must take responsi bility for accuracy! Many hands and heads have helped to make this book. I thank all my colleagues past and present for their enduring though critical support, and I thank with special pleasure: E.]. M. Evesham who fashioned the diagrams;]. Free, D.J. Stradling and]. P.E.C. Darlington who supplied photographs; D.Y. Brian and R.A. Weller who were meticulous on the linguistic side; and G. Frith and R.M. Jones who collated the references. List of plates 1. Fungus combs of Acromyrmex octospinosus and Macrotermes michaelseni. 13 2. Mouthparts of larval Myrmica; 1 Introduction -- 2 Food -- 2.1 Termites as decomposers -- 2.2 Wasps and ants as predators -- 2.3 Sugars as fuel save prey -- 2.4 Seed eaters -- 2.5 Leaf eaters -- 2.6 Pollen eaters -- 3 Foraging by individuals -- 3.1 Foraging strategy -- 3.2 Worker variability -- 4 Foraging in groups -- 4.1 Communication about food -- 4.2 Group slave-raiding -- 4.3 Tunnels and tracks -- 4.4 Nomadic foraging -- 5 Cavity nests and soil mounds -- 5.1 Cavities and burrows -- 5.2 Soil mounds -- 6 Nests of fibre, silk and wax -- 6.1 Mounds of vegetation and tree nests -- 6.2 Combs of cells -- 7 Microclimate -- 7.1 Environmental regulation -- 7.2 Metabolic regulation -- 8 Defence -- 8.1 Painful and paralysing injections -- 8.2 Toxic smears and repellants -- 9 Food processing -- 9.1 Mastication, extraction and regurgitation -- 9.2 Yolk food supplements -- 9.3 Head food glands -- 10 Early population growth -- 10.1 Food distribution -- 10.2 Colony foundation -- 10.3 The growth spurt -- 11 Maturation -- 11.1 Simple models of reproduction -- 11.2 Social control over caste -- 11.3 Males in social Hymenoptera -- 11.4 Maturation in general -- 12 Reproduction -- 12.1 Caste morphogenesis -- 12.2 Copulation and dispersal -- 12.3 Production -- 12.4 Summary -- 13 Evolution of insect societies -- 13.1 Theories of individual selection -- 13.2 Models of these theories -- 13.3 Group selection -- 13.4 Conclusions -- 14 Colonies -- 14.1 The colony barrier -- 14.2 Queen number and species ecology -- 14.3 Queen interaction and queen relatedness -- 15 Comparative ecology of congeneric species -- 15.1 Ant and termite races -- 15.2 Desert ants and termites -- 15.3 Ants and termites in grassland -- 15.4 Forest ants and termites -- 15.5 Wasps and bumblebees -- 15.6 Advanced bees -- 16 Communities -- 16.1 Temperate zone communities in grass and woodland -- 16.2 Desert communities -- 16.3 Tropical rain forest -- 16.4 Conclusions -- 17 Two themes -- 17.1 Plant mutualism -- 17.2 Social organization -- References -- Author index

The Ecological Theatre of Selfish Elements
Abstract. Some selfish genetic elements enhance their transmission to the next generation by interfering with and eliminating competing variants within the

Biological Sex is a social construct
I recently tweeted, as an aside, that biological sex is a social construct, and the backlash and attacks were swift, incredulous and heavily reliant upon very basic biology. There is a common perce…

PENiS | Notion
male reproductive system Organs of the male reproductive system.

What’s Earth’s dominant species by mass?
You might have heard that all the ants in the world weigh as much combined as all the humans. That isn’t true. We outweigh ants 5 to 1.1 Termites might have us beat, though.2 Either way, it’s not r…
Symbiotic organs in insects: diversity, functional implications, and terminology
Abstract With over a million described species, insects represent the most successful group of animals on Earth. One of the drivers of insect diversity is their ability to engage in multifold beneficial symbioses with microorganisms, often involving specialized host organs to accommodate intra- or extracellular symbionts. The existence of such organs and their importance for sustaining and transmitting beneficial symbionts has been known for over a century, and specific terms have been established for categorizing organs harbouring intracellular bacteria (bacteriomes) or fungi (mycetomes), or cuticular crypts containing extracellular fungi (mycetangia). For others, however, general terms are lacking, e.g. organs containing extracellular bacteria associated with the cuticle or with the digestive tract. Furthermore, previously established terms have been misused in other contexts. Notably, ‘bacteriome’ has been increasingly employed in the microbiome field to refer to bacterial communities, instead of the term’s original meaning of specialized organs housing intracellular bacterial symbionts. Here, we review and categorize the diversity of symbiotic organs in insects and propose a unified terminology. Our hope is that this common language will facilitate communication and thereby support the field of symbiosis research in unravelling commonalities and differences in the evolution, ecology, development, physiology and molecular basis across symbiotic interactions. This article is part of the theme issue ‘Life in natural microcosms’.

The ultrasocial origin of the Anthropocene
The current geological epoch has been dubbed the Anthropocene—the age of humans. We argue that the roots of the Anthropocene lie in the agricultural revolution that began some 8000years ago. Unique human psychological and cultural characteristics were present in our distant hunter–gatherer past, but in terms of the biophysical impact of our species, agricultural represented an unequivocal and decisive evolutionary break. With the transition to agriculture human society began to function as a superorganism functioning as a single unit designed by social natural selection to produce economic surplus. Where environmental conditions were permitted, early human agricultural societies followed the same pattern as a few social insects and exhibited explosive population growth, complex and detailed division of labor, intensive resource exploitation, territorial expansion, and a social organization favoring the survival and growth of the supergroup over the well-being of individuals within the group. Similar economic forces lie behind ultrasociality in social insects and humans—increased productivity from the division of labor, increasing returns to scale, and the exploitation of stocks of productive resources. Exploring the evolutionary mechanisms behind ultrasociality offers insights into the growth imperative that threatens the stability of the earth's life support systems.
Nymph (biology)
In biology, a nymph is the juvenile form of some invertebrates, particularly insects, which undergoes gradual metamorphosis (hemimetabolism) before reaching its adult stage. Unlike a typical larva, a nymph's overall form already resembles that of the adult, except for a lack of wings and the emergence of genitalia. In addition, while a nymph moults, it never enters a pupal stage. Instead, the final moult results in an adult insect. Nymphs undergo multiple stages of development called instars.

VULVA | Notion
— Female reproductive system Organs of the human female reproductive system.

Social Constructs (or, 'What is A Woman, Really?')
Evolution
Evolution is the change in the heritable characteristics of biological populations over successive generations. It occurs when evolutionary processes such as genetic drift and natural selection act on genetic variation, resulting in certain characteristics becoming more or less common within a population over successive generations. The process of evolution has given rise to biodiversity at every level of biological organisation.
